Rice Science ›› 2026, Vol. 33 ›› Issue (5): 715-734.DOI: 10.1016/j.rsci.2026.06.002
• Research Papers • Previous Articles
Wonjae Hwang1, Sunok Moon1, Ki-Hong Jung1,2( )
Received:2026-03-02
Accepted:2026-06-02
Online:2026-09-28
Published:2026-09-30
Contact:
Ki-Hong Jung (khjung2010@khu.ac.kr)
Wonjae Hwang, Sunok Moon, Ki-Hong Jung. RE3DB: A Multi-Omics Phylogenomics Platform for Rice E3 Ubiquitin-Ligase-System Genes and Candidate F-Box Genes Associated with Pollen Germination[J]. Rice Science, 2026, 33(5): 715-734.
Add to citation manager EndNote|Ris|BibTeX
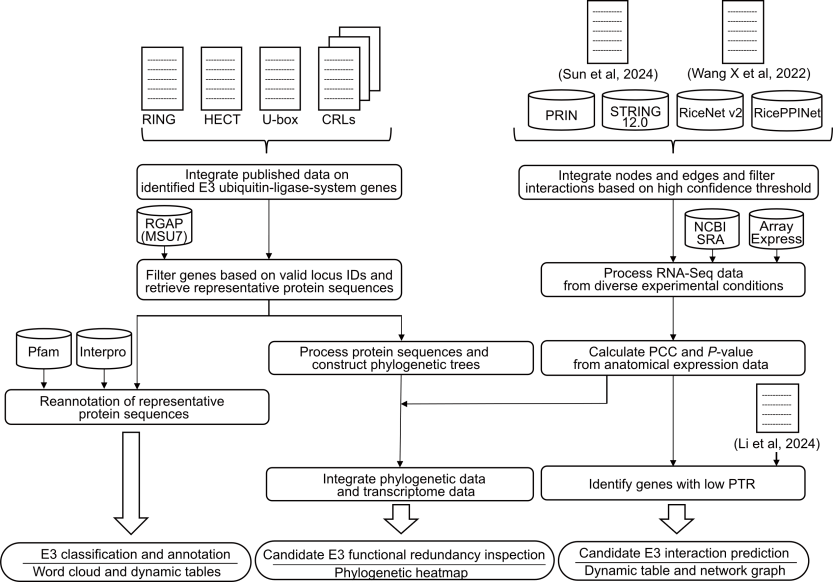
Fig. 1. Overview of RE3DB data integration and interactive modules. RE3DB integrates curated rice E3 ubiquitin-ligase-system gene annotations, protein-protein interaction (PPI) resources, RNA sequencing (RNA-seq) expression profiles, protein-to-transcript ratio (PTR) data, and family-level phylogenies. The platform contains three interactive modules: classification and annotation, phylogeny-guided redundancy prioritization, and E3 interaction prediction. Main outputs include family-level summaries, downloadable gene annotation tables, phylogenetic heatmaps, and E3-centered interaction networks. RING, Really Interesting New Gene; HECT, Homologous to E6AP C-terminus; CRL, Cullin-RING ligase; RGAP, Rice Genome Annotation Project; SRA, Sequence Read Archive; PCC, Pearson correlation coefficient.
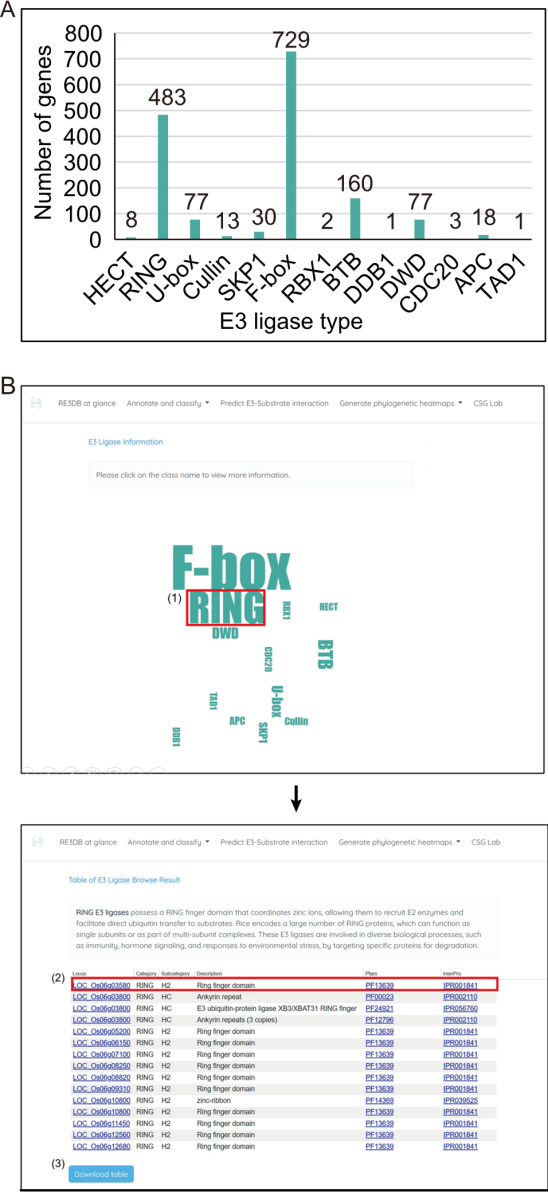
Fig. 2. Classification and annotation of rice E3-system genes in RE3DB. A, Word-cloud view of curated rice E3-system families. Font size is proportional to the number of genes in each family. B, Family-specific annotation table showing Rice Genome Annotation Project (RGAP, MSU7) locus identifiers, E3 family and subfamily, functional role category, Pfam-based description, Pfam entry, and InterPro entry. Hyperlinked locus identifiers connect to RGAP gene pages, and Pfam or InterPro entries connect to the corresponding domain pages. OsBBI1 (BLAST AND BTH-INDUCED 1; LOC_Os06g03580) is highlighted as an example. The download button exports the displayed table as a CSV file. APC, Anaphase-promoting complex; BTB, Broad-complex, tramtrack and bric-à-brac; CDC20, Cell division cycle 20; DDB1, DNA damage-binding protein 1; DWD, DDB1-binding WD40; HECT, Homologous to E6AP C-terminus; RBX1, RING box protein 1; RING, Really Interesting New Gene; SKP1, S-phase kinase-associated protein 1; TAD1, Tiller Angle Control 1.
| E3 system category | E3 family | E3 sub-family | No. of genes identified |
|---|---|---|---|
| Catalytic E3 ligase proteins or catalytic subunits | HECT | 8 | |
| RING | C2 | 1 | |
| H2 | 278 | ||
| HC | 118 | ||
| Not determined | 63 | ||
| V | 23 | ||
| U-box | I | 1 | |
| II | 28 | ||
| III | 16 | ||
| IV | 16 | ||
| V | 7 | ||
| VI | 2 | ||
| VII | 6 | ||
| VIII | 1 | ||
| RBX1 | 2 | ||
| Substrate-recognition or specificity components | F-box | FBA | 4 |
| FBD | 17 | ||
| FBDUF | 63 | ||
| FBK | 25 | ||
| FBL | 61 | ||
| FBLD | 9 | ||
| FBO | 24 | ||
| FBT | 14 | ||
| FBW | 2 | ||
| FBX | 458 | ||
| Not determined | 52 | ||
| BTB | 160 | ||
| DWD | A | 27 | |
| B | 11 | ||
| C | 12 | ||
| D | 17 | ||
| E | 1 | ||
| I | 1 | ||
| J | 1 | ||
| K | 1 | ||
| L | 4 | ||
| M | 1 | ||
| N | 1 | ||
| CDC20 | 3 | ||
| TAD1 | 1 | ||
| Linker/adaptor-core components | DDB1 | 1 | |
| SKP1 | 30 | ||
| Scaffold/platform components | Cullin | Cullin 1a-1 | 1 |
| Cullin 1a | 1 | ||
| Cullin 1b | 1 | ||
| Cullin 1c | 1 | ||
| Cullin 1d | 1 | ||
| Cullin 1e | 1 | ||
| Cullin 1f | 1 | ||
| Cullin 3a | 1 | ||
| Cullin 3b like | 1 | ||
| Cullin 3b | 1 | ||
| Cullin 3c | 1 | ||
| Cullin 4 | 1 | ||
| Not determined | 1 | ||
| Functionally heterogeneous complex | APC | 18 |
Table 1. Classification of rice E3-system genes in RE3DB.
| E3 system category | E3 family | E3 sub-family | No. of genes identified |
|---|---|---|---|
| Catalytic E3 ligase proteins or catalytic subunits | HECT | 8 | |
| RING | C2 | 1 | |
| H2 | 278 | ||
| HC | 118 | ||
| Not determined | 63 | ||
| V | 23 | ||
| U-box | I | 1 | |
| II | 28 | ||
| III | 16 | ||
| IV | 16 | ||
| V | 7 | ||
| VI | 2 | ||
| VII | 6 | ||
| VIII | 1 | ||
| RBX1 | 2 | ||
| Substrate-recognition or specificity components | F-box | FBA | 4 |
| FBD | 17 | ||
| FBDUF | 63 | ||
| FBK | 25 | ||
| FBL | 61 | ||
| FBLD | 9 | ||
| FBO | 24 | ||
| FBT | 14 | ||
| FBW | 2 | ||
| FBX | 458 | ||
| Not determined | 52 | ||
| BTB | 160 | ||
| DWD | A | 27 | |
| B | 11 | ||
| C | 12 | ||
| D | 17 | ||
| E | 1 | ||
| I | 1 | ||
| J | 1 | ||
| K | 1 | ||
| L | 4 | ||
| M | 1 | ||
| N | 1 | ||
| CDC20 | 3 | ||
| TAD1 | 1 | ||
| Linker/adaptor-core components | DDB1 | 1 | |
| SKP1 | 30 | ||
| Scaffold/platform components | Cullin | Cullin 1a-1 | 1 |
| Cullin 1a | 1 | ||
| Cullin 1b | 1 | ||
| Cullin 1c | 1 | ||
| Cullin 1d | 1 | ||
| Cullin 1e | 1 | ||
| Cullin 1f | 1 | ||
| Cullin 3a | 1 | ||
| Cullin 3b like | 1 | ||
| Cullin 3b | 1 | ||
| Cullin 3c | 1 | ||
| Cullin 4 | 1 | ||
| Not determined | 1 | ||
| Functionally heterogeneous complex | APC | 18 |
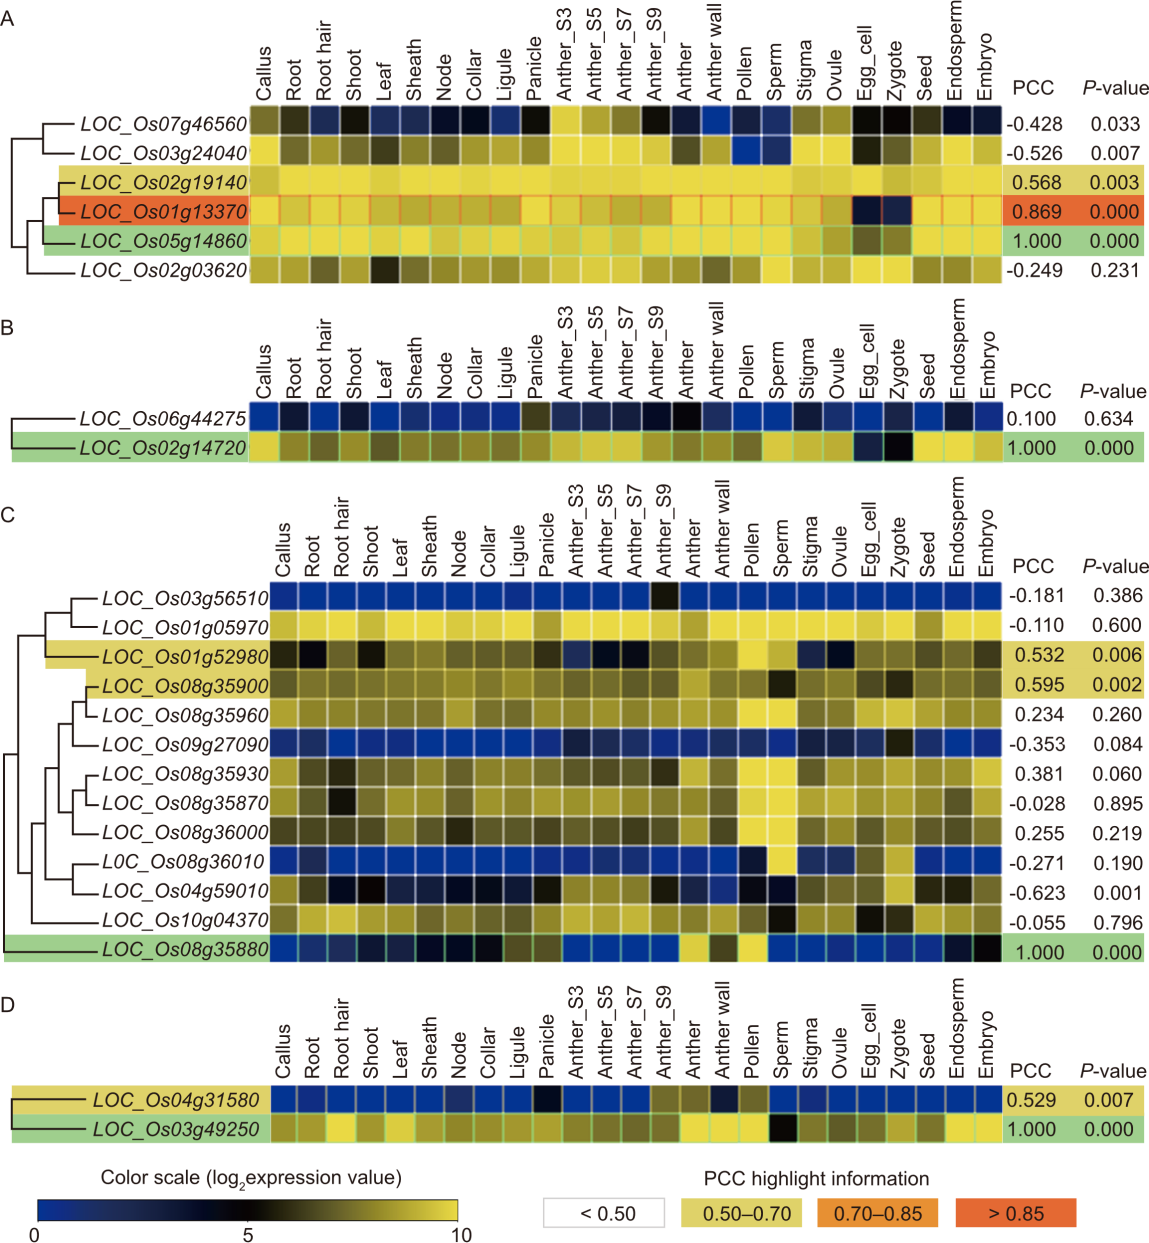
Fig. 3. Phylogenetic heatmaps for redundancy-aware prioritization of rice E3-system genes. A, RIP1-RIP6 RING-type E3 clade, a previously validated redundant gene set. B, GW2 (LOC_Os02g14720), a RING-type E3 gene known to act as a major grain-size regulator. C, LOC_Os10g04370, a mature-anther-preferential F-box candidate prioritized as a single-locus exploratory example. D, LOC_Os03g49250, a mature-anther-preferential F-box candidate whose local clade includes LOC_Os04g31580 as a possible companion paralog for future testing. RE3DB overlays transcript abundance across 25 rice tissues onto family-level protein phylogenies. For single-gene queries, Pearson correlation coefficients (PCCs) and raw two-tailed Pearson correlation P-values are shown for neighboring genes relative to the query locus.
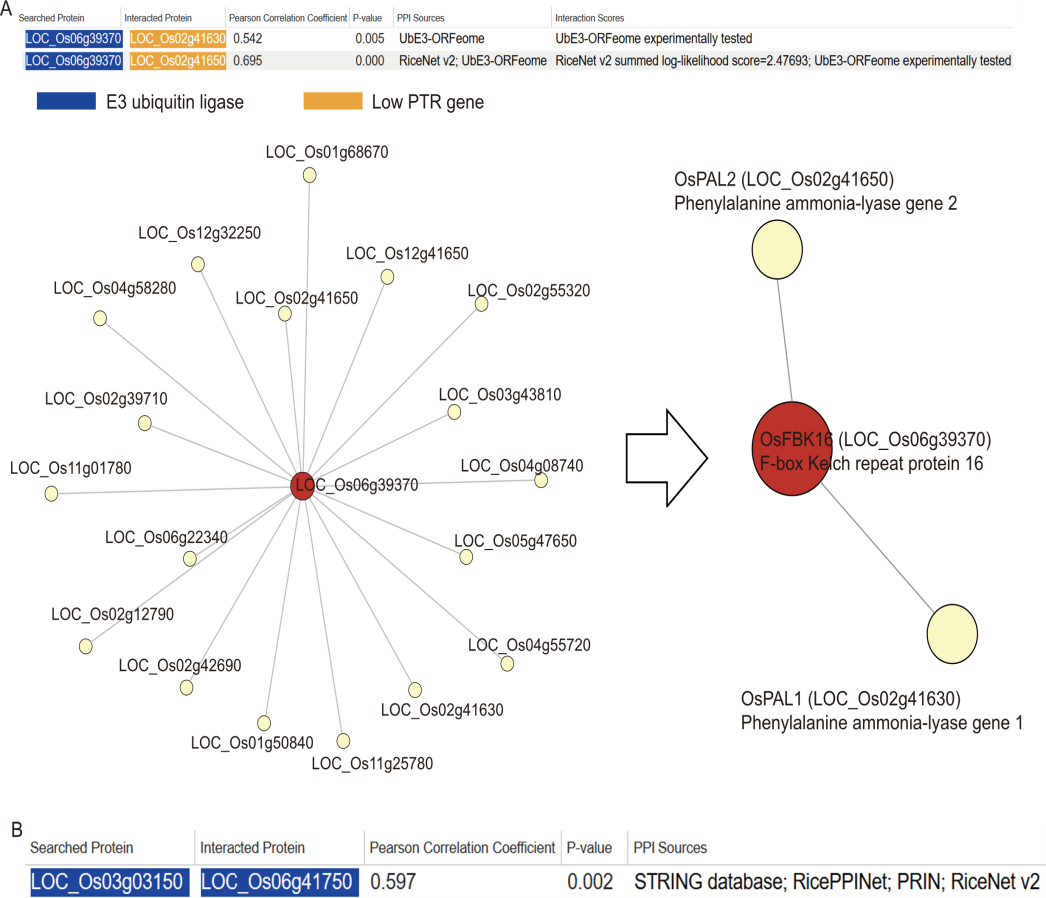
Fig. 4. Integrated evidence for E3 interaction prediction in RE3DB. A, Querying OsFBK16 (LOC_Os06g39370) returns predicted interacting proteins, including OsPAL1 (LOC_Os02g41630) and OsPAL2 (LOC_Os02g41650), which were previously supported as OsFBK16-associated proteins. B, Querying TAD1/TE (LOC_Os03g03150), a Cdh1/CCS52-type anaphase-promoting complex (APC) activator, returns OsCDC27 (LOC_ Os06g41750), an APC core subunit, as a multi-source-supported E3-complex interaction. RE3DB predicts E3-centered interactions by combining high-confidence protein-protein interaction (PPI) resources, transcript co-expression across 25 tissues, raw Pearson correlation coefficient (PCC)-associated P-values, and low protein-to-transcript ratio (PTR) information across 14 tissues. The output table reports supporting PPI sources, source-specific scores, PCC, raw P-value, and tissues with low PTR, rather than converting heterogeneous source scores into a single composite score.
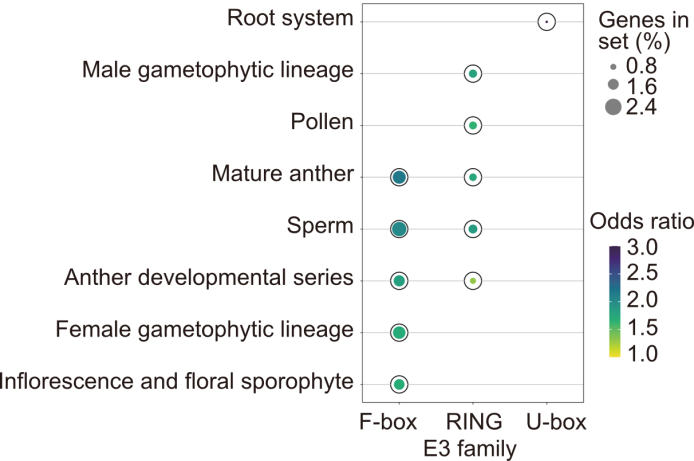
Fig. 5. Enrichment of tissue-preferential E3-system families. For each E3-system family, the top enriched anatomical terms ranked by odds ratio and passing false-discovery-rate (FDR)-adjusted P ≤ 0.05 are shown. Dot size indicates the percentage of tissue-preferential family members assigned to each term, and dot color indicates the odds ratio. Because E3-system families differ greatly in size, enrichment should be interpreted using odds ratios and FDR-adjusted P-values rather than raw gene counts alone. Complete tissue-preferential gene lists are provided in Tables S6 and S7, and family-specific expression profiles are shown in Figs. S3-S12. RING, Really Interesting New Gene.
| Locus ID | RUPO | OSMTD2 | GORI | MADSTRI | TAPE | OSRAC6 | RALF17/19 | ABCG16/28 | GTRD5 | GROUP |
|---|---|---|---|---|---|---|---|---|---|---|
| LOC_Os06g35080 | O | RAD | ||||||||
| LOC_Os09g06620 | O | O | GD/RAD | |||||||
| LOC_Os12g05609 | O | M2D | ||||||||
| LOC_Os12g27790 | O | O | M2D/RAD | |||||||
| LOC_Os11g38180 | O | O | O | M2D/R6D/RAD | ||||||
| LOC_Os01g40160 | O | O | O | O | O | O | RD/M2D/GD/MD/R6D/AD | |||
| LOC_Os02g52230 | O | MD | ||||||||
| LOC_Os09g28120 | O | MD | ||||||||
| LOC_Os01g71450 | O | MD | ||||||||
| LOC_Os04g35190 | O | MD | ||||||||
| LOC_Os03g50050 | O | MD | ||||||||
| LOC_Os04g40330 | O | MD | ||||||||
| LOC_Os12g40140 | O | MD | ||||||||
| LOC_Os03g46530 | O | MD | ||||||||
| LOC_Os03g25250 | O | MD | ||||||||
| LOC_Os01g56750 | O | MD | ||||||||
| LOC_Os04g57290 | O | MD | ||||||||
| LOC_Os01g17390 | O | MD | ||||||||
| LOC_Os03g12190 | O | MD | ||||||||
| LOC_Os08g35880 | O | MD | ||||||||
| LOC_Os03g36439 | O | MD | ||||||||
| LOC_Os11g38130 | O | MD | ||||||||
| LOC_Os01g06360 | O | O | O | RD/MD/TD | ||||||
| LOC_Os09g17190 | O | O | O | O | RD/GD/MD/TD | |||||
| LOC_Os04g11450 | O | O | O | RD/GD/MD | ||||||
| LOC_Os04g42670 | O | O | RD/MD | |||||||
| LOC_Os03g49250 | O | O | RD/MD | |||||||
| LOC_Os05g46320 | O | O | RD/MD | |||||||
| LOC_Os02g17210 | O | O | RD/MD | |||||||
| LOC_Os07g09110 | O | O | RD/MD | |||||||
| LOC_Os10g04370 | O | O | RD/MD | |||||||
| LOC_Os02g56820 | O | O | O | MD/R6D/RAD | ||||||
| LOC_Os03g51760 | O | O | MD/R6D | |||||||
| LOC_Os11g38100 | O | O | RD/R6D | |||||||
| LOC_Os03g25240 | O | O | O | RD/MD/R6D | ||||||
| LOC_Os03g25650 | O | O | O | O | RD/MD/R6D/RAD | |||||
| LOC_Os04g40800 | O | O | O | O | O | GD/MD/TD/R6D/G5D | ||||
| LOC_Os08g24830 | O | O | O | GD/MD/R6D | ||||||
| LOC_Os10g10420 | O | O | O | O | RD/GD/MD/R6D | |||||
| LOC_Os05g49540 | O | O | O | O | O | RD/GD/MD/R6D/G5D | ||||
| LOC_Os03g25220 | O | O | RD/RAD | |||||||
| LOC_Os07g03110 | O | RD | ||||||||
| LOC_Os11g42280 | O | RD | ||||||||
| LOC_Os08g09460 | O | RD | ||||||||
| LOC_Os07g18600 | O | RD | ||||||||
| LOC_Os02g19540 | O | RD | ||||||||
| LOC_Os11g42310 | O | RD | ||||||||
| LOC_Os02g33310 | O | RD | ||||||||
| LOC_Os03g46140 | O | RD | ||||||||
| LOC_Os06g02110 | O | RD | ||||||||
| LOC_Os01g55430 | O | RD | ||||||||
| LOC_Os04g19800 | O | RD | ||||||||
| LOC_Os03g25190 | O | RD | ||||||||
| LOC_Os05g08350 | O | RD | ||||||||
| LOC_Os02g03910 | O | RD | ||||||||
| LOC_Os06g41520 | O | RD | ||||||||
| LOC_Os05g25580 | O | RD | ||||||||
| LOC_Os01g33490 | O | RD | ||||||||
| LOC_Os10g06700 | O | RD | ||||||||
| LOC_Os02g28600 | O | O | O | RD/GD/AD | ||||||
| LOC_Os04g31580 | O | O | RD/GD | |||||||
| LOC_Os07g36280 | O | O | O | RD/GD/TD | ||||||
| LOC_Os08g38490 | O | TD | ||||||||
| LOC_Os10g10410 | O | TD | ||||||||
| LOC_Os11g36350 | O | O | O | O | RD/M2D/TD/R6D | |||||
| LOC_Os05g51100 | O | O | O | O | RD/TD/R6D/RAD | |||||
| LOC_Os11g42270 | O | AD | ||||||||
| LOC_Os04g39070 | O | AD | ||||||||
| LOC_Os09g22460 | O | AD | ||||||||
| LOC_Os04g40770 | O | AD | ||||||||
| LOC_Os09g15460 | O | AD | ||||||||
| LOC_Os08g36960 | O | O | AD/G5D | |||||||
| LOC_Os08g09590 | O | O | O | TD/AD/G5D | ||||||
| LOC_Os02g41930 | O | O | O | MD/AD/G5D | ||||||
| LOC_Os04g40960 | O | O | O | O | RD/MD/AD/G5D | |||||
| LOC_Os02g33840 | O | O | O | O | RD/MD/AD/G5D | |||||
| LOC_Os01g71440 | O | O | O | GD/MD/AD | ||||||
| LOC_Os07g36360 | O | O | O | M2D/MD/AD | ||||||
| LOC_Os05g01620 | O | O | MD/AD | |||||||
| LOC_Os03g56450 | O | GD | ||||||||
| LOC_Os03g12200 | O | GD | ||||||||
| LOC_Os01g28520 | O | GD | ||||||||
| LOC_Os08g40640 | O | GD | ||||||||
| LOC_Os09g17152 | O | GD | ||||||||
| LOC_Os02g54550 | O | GD | ||||||||
| LOC_Os02g51350 | O | GD | ||||||||
| LOC_Os07g03090 | O | O | O | M2D/GD/G5D | ||||||
| LOC_Os05g02550 | O | O | GD/G5D | |||||||
| LOC_Os07g48940 | O | O | GD/G5D | |||||||
| LOC_Os10g34340 | O | O | GD/G5D | |||||||
| LOC_Os02g56760 | O | O | RD/G5D | |||||||
| LOC_Os03g47420 | O | O | RD/G5D | |||||||
| LOC_Os03g24200 | O | G5D | ||||||||
| LOC_Os08g27190 | O | G5D | ||||||||
| LOC_Os02g54240 | O | G5D | ||||||||
| LOC_Os07g16800 | O | G5D | ||||||||
| LOC_Os03g46500 | O | G5D | ||||||||
| LOC_Os07g13930 | O | G5D | ||||||||
| LOC_Os08g31690 | O | G5D | ||||||||
| LOC_Os04g26240 | O | G5D | ||||||||
| LOC_Os07g08570 | O | G5D | ||||||||
| LOC_Os02g35530 | O | G5D | ||||||||
| LOC_Os11g33220 | O | G5D | ||||||||
| LOC_Os07g36520 | O | G5D | ||||||||
| LOC_Os04g31540 | O | G5D | ||||||||
| LOC_Os10g10390 | O | G5D | ||||||||
| LOC_Os04g35930 | O | G5D | ||||||||
| LOC_Os02g16760 | O | G5D | ||||||||
| LOC_Os07g36530 | O | R6D | ||||||||
| LOC_Os12g34290 | O | O | O | R6D/RAD/G5D | ||||||
| LOC_Os03g56440 | O | O | R6D/G5D |
Table 2. Downregulated mature-anther-preferential F-box candidates across nine male-sterile mutant backgrounds.
| Locus ID | RUPO | OSMTD2 | GORI | MADSTRI | TAPE | OSRAC6 | RALF17/19 | ABCG16/28 | GTRD5 | GROUP |
|---|---|---|---|---|---|---|---|---|---|---|
| LOC_Os06g35080 | O | RAD | ||||||||
| LOC_Os09g06620 | O | O | GD/RAD | |||||||
| LOC_Os12g05609 | O | M2D | ||||||||
| LOC_Os12g27790 | O | O | M2D/RAD | |||||||
| LOC_Os11g38180 | O | O | O | M2D/R6D/RAD | ||||||
| LOC_Os01g40160 | O | O | O | O | O | O | RD/M2D/GD/MD/R6D/AD | |||
| LOC_Os02g52230 | O | MD | ||||||||
| LOC_Os09g28120 | O | MD | ||||||||
| LOC_Os01g71450 | O | MD | ||||||||
| LOC_Os04g35190 | O | MD | ||||||||
| LOC_Os03g50050 | O | MD | ||||||||
| LOC_Os04g40330 | O | MD | ||||||||
| LOC_Os12g40140 | O | MD | ||||||||
| LOC_Os03g46530 | O | MD | ||||||||
| LOC_Os03g25250 | O | MD | ||||||||
| LOC_Os01g56750 | O | MD | ||||||||
| LOC_Os04g57290 | O | MD | ||||||||
| LOC_Os01g17390 | O | MD | ||||||||
| LOC_Os03g12190 | O | MD | ||||||||
| LOC_Os08g35880 | O | MD | ||||||||
| LOC_Os03g36439 | O | MD | ||||||||
| LOC_Os11g38130 | O | MD | ||||||||
| LOC_Os01g06360 | O | O | O | RD/MD/TD | ||||||
| LOC_Os09g17190 | O | O | O | O | RD/GD/MD/TD | |||||
| LOC_Os04g11450 | O | O | O | RD/GD/MD | ||||||
| LOC_Os04g42670 | O | O | RD/MD | |||||||
| LOC_Os03g49250 | O | O | RD/MD | |||||||
| LOC_Os05g46320 | O | O | RD/MD | |||||||
| LOC_Os02g17210 | O | O | RD/MD | |||||||
| LOC_Os07g09110 | O | O | RD/MD | |||||||
| LOC_Os10g04370 | O | O | RD/MD | |||||||
| LOC_Os02g56820 | O | O | O | MD/R6D/RAD | ||||||
| LOC_Os03g51760 | O | O | MD/R6D | |||||||
| LOC_Os11g38100 | O | O | RD/R6D | |||||||
| LOC_Os03g25240 | O | O | O | RD/MD/R6D | ||||||
| LOC_Os03g25650 | O | O | O | O | RD/MD/R6D/RAD | |||||
| LOC_Os04g40800 | O | O | O | O | O | GD/MD/TD/R6D/G5D | ||||
| LOC_Os08g24830 | O | O | O | GD/MD/R6D | ||||||
| LOC_Os10g10420 | O | O | O | O | RD/GD/MD/R6D | |||||
| LOC_Os05g49540 | O | O | O | O | O | RD/GD/MD/R6D/G5D | ||||
| LOC_Os03g25220 | O | O | RD/RAD | |||||||
| LOC_Os07g03110 | O | RD | ||||||||
| LOC_Os11g42280 | O | RD | ||||||||
| LOC_Os08g09460 | O | RD | ||||||||
| LOC_Os07g18600 | O | RD | ||||||||
| LOC_Os02g19540 | O | RD | ||||||||
| LOC_Os11g42310 | O | RD | ||||||||
| LOC_Os02g33310 | O | RD | ||||||||
| LOC_Os03g46140 | O | RD | ||||||||
| LOC_Os06g02110 | O | RD | ||||||||
| LOC_Os01g55430 | O | RD | ||||||||
| LOC_Os04g19800 | O | RD | ||||||||
| LOC_Os03g25190 | O | RD | ||||||||
| LOC_Os05g08350 | O | RD | ||||||||
| LOC_Os02g03910 | O | RD | ||||||||
| LOC_Os06g41520 | O | RD | ||||||||
| LOC_Os05g25580 | O | RD | ||||||||
| LOC_Os01g33490 | O | RD | ||||||||
| LOC_Os10g06700 | O | RD | ||||||||
| LOC_Os02g28600 | O | O | O | RD/GD/AD | ||||||
| LOC_Os04g31580 | O | O | RD/GD | |||||||
| LOC_Os07g36280 | O | O | O | RD/GD/TD | ||||||
| LOC_Os08g38490 | O | TD | ||||||||
| LOC_Os10g10410 | O | TD | ||||||||
| LOC_Os11g36350 | O | O | O | O | RD/M2D/TD/R6D | |||||
| LOC_Os05g51100 | O | O | O | O | RD/TD/R6D/RAD | |||||
| LOC_Os11g42270 | O | AD | ||||||||
| LOC_Os04g39070 | O | AD | ||||||||
| LOC_Os09g22460 | O | AD | ||||||||
| LOC_Os04g40770 | O | AD | ||||||||
| LOC_Os09g15460 | O | AD | ||||||||
| LOC_Os08g36960 | O | O | AD/G5D | |||||||
| LOC_Os08g09590 | O | O | O | TD/AD/G5D | ||||||
| LOC_Os02g41930 | O | O | O | MD/AD/G5D | ||||||
| LOC_Os04g40960 | O | O | O | O | RD/MD/AD/G5D | |||||
| LOC_Os02g33840 | O | O | O | O | RD/MD/AD/G5D | |||||
| LOC_Os01g71440 | O | O | O | GD/MD/AD | ||||||
| LOC_Os07g36360 | O | O | O | M2D/MD/AD | ||||||
| LOC_Os05g01620 | O | O | MD/AD | |||||||
| LOC_Os03g56450 | O | GD | ||||||||
| LOC_Os03g12200 | O | GD | ||||||||
| LOC_Os01g28520 | O | GD | ||||||||
| LOC_Os08g40640 | O | GD | ||||||||
| LOC_Os09g17152 | O | GD | ||||||||
| LOC_Os02g54550 | O | GD | ||||||||
| LOC_Os02g51350 | O | GD | ||||||||
| LOC_Os07g03090 | O | O | O | M2D/GD/G5D | ||||||
| LOC_Os05g02550 | O | O | GD/G5D | |||||||
| LOC_Os07g48940 | O | O | GD/G5D | |||||||
| LOC_Os10g34340 | O | O | GD/G5D | |||||||
| LOC_Os02g56760 | O | O | RD/G5D | |||||||
| LOC_Os03g47420 | O | O | RD/G5D | |||||||
| LOC_Os03g24200 | O | G5D | ||||||||
| LOC_Os08g27190 | O | G5D | ||||||||
| LOC_Os02g54240 | O | G5D | ||||||||
| LOC_Os07g16800 | O | G5D | ||||||||
| LOC_Os03g46500 | O | G5D | ||||||||
| LOC_Os07g13930 | O | G5D | ||||||||
| LOC_Os08g31690 | O | G5D | ||||||||
| LOC_Os04g26240 | O | G5D | ||||||||
| LOC_Os07g08570 | O | G5D | ||||||||
| LOC_Os02g35530 | O | G5D | ||||||||
| LOC_Os11g33220 | O | G5D | ||||||||
| LOC_Os07g36520 | O | G5D | ||||||||
| LOC_Os04g31540 | O | G5D | ||||||||
| LOC_Os10g10390 | O | G5D | ||||||||
| LOC_Os04g35930 | O | G5D | ||||||||
| LOC_Os02g16760 | O | G5D | ||||||||
| LOC_Os07g36530 | O | R6D | ||||||||
| LOC_Os12g34290 | O | O | O | R6D/RAD/G5D | ||||||
| LOC_Os03g56440 | O | O | R6D/G5D |
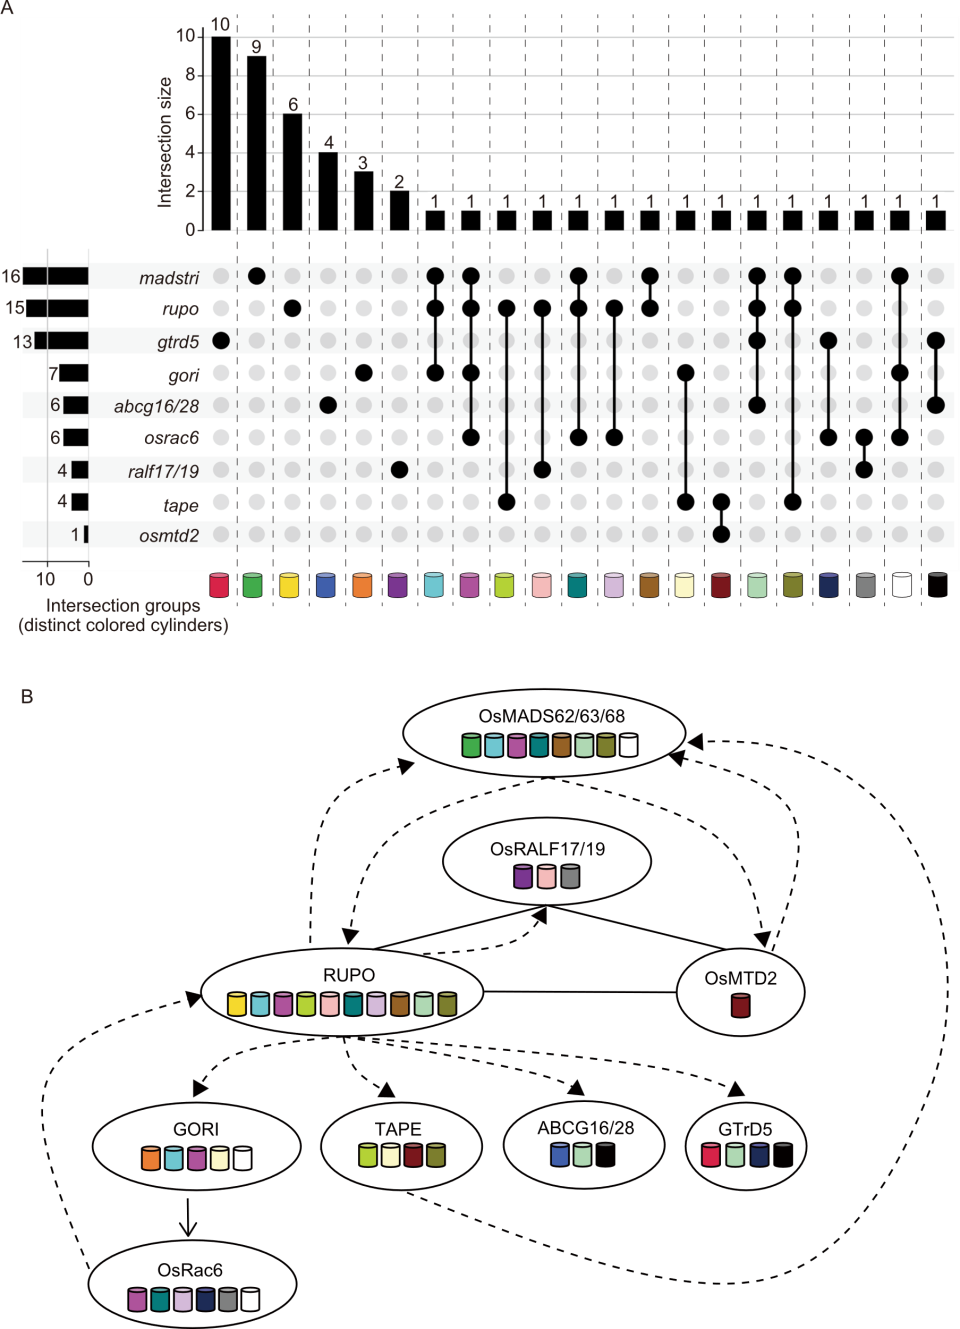
Fig. 6. Prioritization of mature-anther-preferential F-box candidates associated with rice pollen germination. A, UpSet plot of mature-anther-preferential F-box genes that were stringently downregulated, defined as log2(fold change) ≤ -2, in nine male-sterile mutant backgrounds affecting pollen germination or pollen-tube growth. Matrix dots indicate the mutant backgrounds included in each intersection group. Vertical cylinders show the number of candidate genes in each intersection, and horizontal bars show the total number of candidates in each mutant set. Distinct cylinder colors identify intersection groups; they do not indicate fold-change magnitude or statistical significance. Matching hex color codes are provided in Table S10. B, Hypothesis-generating network integrating stringently downregulated F-box candidates with literature-curated pollen-germination regulators. Solid edges indicate experimentally supported regulatory relationships or protein-protein interactions, whereas dotted edges indicate inferred associations based on shared downregulation patterns in RNA-seq data.
| [1] | Bielskienė K, Bagdonienė L, Mozūraitienė J, et al. 2015. E3 ubiquitin ligases as drug targets and prognostic biomarkers in melanoma. Medicina, 51(1): 1-9. |
| [2] | Blum M, Andreeva A, Florentino L C, et al. 2025. InterPro: The protein sequence classification resource in 2025. Nucleic Acids Res, 53(D1): D444-D456. |
| [3] | Chang S W, Huang G Q, Wang D X, et al. 2022. Rice SIAH E3 ligases interact with RMD formin and affect plant morphology. Rice, 15(1): 6. |
| [4] | Cock P J A, Antao T, Chang J T, et al. 2009. Biopython: Freely available Python tools for computational molecular biology and bioinformatics. Bioinformatics, 25(11): 1422-1423. |
| [5] | Craig A, Ewan R, Mesmar J, et al. 2009. E3 ubiquitin ligases and plant innate immunity. J Exp Bot, 60(4): 1123-1132. |
| [6] | Eloy N B, de Freitas Lima M, Ferreira P C G, et al. 2015. The role of the anaphase-promoting complex/cyclosome in plant growth. Crit Rev Plant Sci, 34(5): 487-505. |
| [7] | Fang Z Q, Liu X Y, Peltz G. 2023. GSEApy: A comprehensive package for performing gene set enrichment analysis in Python. Bioinformatics, 39(1): btac757. |
| [8] | Gu H B, Zhu P C, Jiao Y M, et al. 2011. PRIN: A predicted rice interactome network. BMC Bioinform, 12(1): 161. |
| [9] | Guindon S, Dufayard J F, Lefort V, et al. 2010. New algorithms and methods to estimate maximum-likelihood phylogenies: Assessing the performance of PhyML 3.0. Syst Biol, 59(3): 307-321. |
| [10] | Hagberg A A, Schult D A, Swart P J. 2008. Exploring network structure, dynamics, and function using NetworkX. In: Varoquaux G, Vaught T, Millman J. Proceedings of the 7th Python in Science Conference. California, the United States: SciPy: 11-15. |
| [11] | Hamilton J P, Li C X, Buell C R. 2025. The rice genome annotation project: An updated database for mining the rice genome. Nucleic Acids Res, 53(D1): D1614-D1622. |
| [12] | Harris C R, Millman K J, van der Walt S J, et al. 2020. Array programming with NumPy. Nature, 585: 357-362. |
| [13] | Hoang D T, Chernomor O, von Haeseler A, et al. 2018. UFBoot2: Improving the ultrafast bootstrap approximation. Mol Biol Evol, 35(2): 518-522. |
| [14] | Hong W J, Kim Y J, Kim E J, et al. 2020. CAFRI-Rice: CRISPR applicable functional redundancy inspector to accelerate functional genomics in rice. Plant J, 104(2): 532-545. |
| [15] | Huerta-Cepas J, Serra F, Bork P. 2016. ETE 3: Reconstruction, analysis, and visualization of phylogenomic data. Mol Biol Evol, 33(6): 1635-1638. |
| [16] | Hunter J D. 2007. Matplotlib: A 2D graphics environment. Comput Sci Eng, 9(3): 90-95. |
| [17] | Hwang W, Hong W J, Kim E J, et al. 2024. The rice online expression profiles array database version 2 (ROADv2): An interactive atlas for rice functional genomics. Rice, 17(1): 75. |
| [18] | Ishibashi T, Kimura S, Yamamoto T, et al. 2003. Rice UV-damaged DNA binding protein homologues are most abundant in proliferating tissues. Gene, 308: 79-87. |
| [19] | Jain M, Nijhawan A, Arora R, et al. 2007. F-box proteins in rice. Genome-wide analysis, classification, temporal and spatial gene expression during panicle and seed development, and regulation by light and abiotic stress. Plant Physiol, 143(4): 1467-1483. |
| [20] | Jones P, Binns D, Chang H Y, et al. 2014. InterProScan 5: Genome-scale protein function classification. Bioinformatics, 30(9): 1236-1240. |
| [21] | Kahloul S, El Beji I H, Boulaflous A, et al. 2013. Structural, expression and interaction analysis of rice SKP1-like genes. DNA Res, 20(1): 67-78. |
| [22] | Kalyaanamoorthy S, Minh B Q, Wong T K F, et al. 2017. ModelFinder: Fast model selection for accurate phylogenetic estimates. Nat Meth, 14(6): 587-589. |
| [23] | Katoh K, Standley D M. 2013. MAFFT multiple sequence alignment software version 7: Improvements in performance and usability. Mol Biol Evol, 30(4): 772-780. |
| [24] | Katoh K, Misawa K, Kuma K, et al. 2002. MAFFT: A novel method for rapid multiple sequence alignment based on fast Fourier transform. Nucleic Acids Res, 30(14): 3059-3066. |
| [25] | Kelley D R. 2018. E3 ubiquitin ligases: Key regulators of hormone signaling in plants. Mol Cell Proteom, 17(6): 1047-1054. |
| [26] | Kim D, Paggi J M, Park C, et al. 2019. Graph-based genome alignment and genotyping with HISAT2 and HISAT-genotype. Nat Biotechnol, 37(8): 907-915. |
| [27] | Kim E J, Hong W J, Kim Y J, et al. 2022. Transcriptome analysis of triple mutant for OsMADS62, OsMADS63, and OsMADS 68 reveals the downstream regulatory mechanism for pollen germination in rice (Oryza sativa). Int J Mol Sci, 23(1): 239. |
| [28] | Kim E J, Kim J H, Hong W J, et al. 2023. Rice pollen-specific OsRALF17 and OsRALF19 are essential for pollen tube growth. J Integr Plant Biol, 65(9): 2218-2236. |
| [29] | Kim E J, Hong W J, Kim Y J, et al. 2025. Global identification of key genes for pollen germination in rice through high-throughput screening and gene editing. J Integr Plant Biol, 67(6): 1665-1684. |
| [30] | Kim J H, Son Y J, Kim E J, et al. 2025. Pollen tube-expressed RUPO forms a complex with OsMTD2 and OsRALF17 and OsRALF19 peptides in rice (Oryza sativa). J Plant Physiol, 305: 154421. |
| [31] | Kim Y J, Jung K H. 2023. WD40-domain protein GORI is an integrative scaffold that is required for pollen tube growth in rice. Plant Signal Behav, 18(1): 2082678. |
| [32] | Kwon Y T, Ciechanover A. 2017. The ubiquitin code in the ubiquitin-proteasome system and autophagy. Trends Biochem Sci, 42(11): 873-886. |
| [33] | Lee J H, Terzaghi W, Gusmaroli G, et al. 2008. Characterization of Arabidopsis and rice DWD proteins and their roles as substrate receptors for CUL4-RING E 3 ubiquitin ligases. Plant Cell, 20(1): 152-167. |
| [34] | Lee T, Oh T, Yang S M, et al. 2015. RiceNet v2: An improved network prioritization server for rice genes. Nucleic Acids Res, 43(W1): W122-W127. |
| [35] | Leek J T, Scharpf R B, Bravo H C, et al. 2010. Tackling the widespread and critical impact of batch effects in high-throughput data. Nat Rev Genet, 11(10): 733-739. |
| [36] | Lex A, Gehlenborg N, Strobelt H, et al. 2014. UpSet: Visualization of intersecting sets. IEEE Trans Vis Comput Graph, 20(12): 1983-1992. |
| [37] | Li S C, Li W B, Huang B, et al. 2013. Natural variation in PTB1 regulates rice seed setting rate by controlling pollen tube growth. Nat Commun, 4: 2793. |
| [38] | Li S T, Ke Y Z, Zhu Y K, et al. 2024. Mass spectrometry-based proteomic landscape of rice reveals a post-transcriptional regulatory role of N6-methyladenosine. Nat Plants, 10(8): 1201-1214. |
| [39] | Li Z Y, Chen S Y, Jhong J H, et al. 2021. UbiNet 2.0:A verified, classified, annotated and updated database of E 3 ubiquitin ligase-substrate interactions. Database, 2021: baab010. |
| [40] | Liao Y, Smyth G K, Shi W. 2014. featureCounts: An efficient general purpose program for assigning sequence reads to genomic features. Bioinformatics, 30(7): 923-930. |
| [41] | Lim S D, Yim W C, Moon J C, et al. 2010. A gene family encoding RING finger proteins in rice: Their expansion, expression diversity, and co-expressed genes. Plant Mol Biol, 72(4): 369-380. |
| [42] | Lin Q B, Wang D, Dong H, et al. 2012. Rice APC/CTE controls tillering by mediating the degradation of MONOCULM 1. Nat Commun, 3: 752. |
| [43] | Lin Y N, Jiang C K, Cheng Z K, et al. 2022. Rice Cell Division Cycle 20s are required for faithful chromosome segregation and cytokinesis during meiosis. Plant Physiol, 188(2): 1111-1128. |
| [44] | Liu J P, Zhang C C, Wei C C, et al. 2016. The RING finger ubiquitin E3 ligase OsHTAS enhances heat tolerance by promoting H2O2-induced stomatal closure in rice. Plant Physiol, 170(1): 429-443. |
| [45] | Liu L H, Damerell D R, Koukouflis L, et al. 2019. UbiHub: A data hub for the explorers of ubiquitination pathways. Bioinformatics, 35(16): 2882-2884. |
| [46] | Liu Q N, Ning Y S, Zhang Y X, et al. 2017. OsCUL3a negatively regulates cell death and immunity by degrading OsNPR1 in rice. Plant Cell, 29(2): 345-359. |
| [47] | Liu S W, Liu Y H, Zhao J W, et al. 2017. A computational interactome for prioritizing genes associated with complex agronomic traits in rice (Oryza sativa). Plant J, 90(1): 177-188. |
| [48] | Love M I, Huber W, Anders S. 2014. Moderated estimation of fold change and dispersion for RNA-seq data with DESeq2. Genome Biol, 15(12): 550. |
| [49] | Marín I. 2013. Evolution of plant HECT ubiquitin ligases. PLoS One, 8(7): e68536. |
| [50] | Martin M. 2011. Cutadapt removes adapter sequences from high-throughput sequencing reads. EMBnet J, 17(1): 10. |
| [51] | McKinney W. 2010. Data structures for statistical computing in Python. In: Proceedings of the Python in Science Conference. Austin, Texas, the United States: SciPy: 56-61. |
| [52] | Medvar B, Raghuram V, Pisitkun T, et al. 2016. Comprehensive database of human E3 ubiquitin ligases:Application to aquaporin-2 regulation. Physiol Genom, 48(7): 502-512. |
| [53] | Minh B Q, Schmidt H A, Chernomor O, et al. 2020. IQ-TREE 2: New models and efficient methods for phylogenetic inference in the genomic era. Mol Biol Evol, 37(5): 1530-1534. |
| [54] | Moin M, Bakshi A, Madhav M S, et al. 2019. Comprehensive expression profiling reveals the possible involvement of Cullins in developmental and stress regulation in rice. Environ Exp Bot, 160: 101-111. |
| [55] | Nandi D, Tahiliani P, Kumar A, et al. 2006. The ubiquitin-proteasome system. J Biosci, 31(1): 137-155. |
| [56] | Ning Y S, Jantasuriyarat C, Zhao Q Z, et al. 2011. The SINA E3 ligase OsDIS1 negatively regulates drought response in rice. Plant Physiol, 157(1): 242-255. |
| [57] | Park G G, Park J J, Yoon J, et al. 2010. A RING finger E3 ligase gene, Oryza sativa Delayed Seed Germination 1 (OsDSG1), controls seed germination and stress responses in rice. Plant Mol Biol, 74(4): 467-478. |
| [58] | Park J J, Yi J, Yoon J, et al. 2011. OsPUB15, an E3 ubiquitin ligase, functions to reduce cellular oxidative stress during seedling establishment. Plant J, 65(2): 194-205. |
| [59] | Paysan-Lafosse T, Andreeva A, Blum M, et al. 2025. The Pfam protein families database: Embracing AI/ML. Nucleic Acids Res, 53(D1): D523-D534. |
| [60] | Pei J M, Andreeva A, Chuguransky S, et al. 2024. Bridging the gap between sequence and structure classifications of proteins with AlphaFold models. J Mol Biol, 436(22): 168764. |
| [61] | Price M N, Dehal P S, Arkin A P. 2010. FastTree 2: Approximately maximum-likelihood trees for large alignments. PLoS One, 5(3): e9490. |
| [62] | Sadanandom A, Bailey M, Ewan R, et al. 2012. The ubiquitin-proteasome system: Central modifier of plant signalling. New Phytol, 196(1): 13-28. |
| [63] | Sampson C, Wang Q P, Otkur W, et al. 2023. The roles of E3 ubiquitin ligases in cancer progression and targeted therapy. Clin Transl Med, 13(3): e1204. |
| [64] | Shalmani A, Huang Y B, Chen Y B, et al. 2021. The highly interactive BTB domain targeting other functional domains to diversify the function of BTB proteins in rice growth and development. Int J Biol Macromol, 192: 1311-1324. |
| [65] | Shu K, Yang W Y. 2017. E3 ubiquitin ligases: Ubiquitous actors in plant development and abiotic stress responses. Plant Cell Physiol, 58(9): 1461-1476. |
| [66] | Song X J, Huang W, Shi M, et al. 2007. A QTL for rice grain width and weight encodes a previously unknown RING-type E3 ubiquitin ligase. Nat Genet, 39(5): 623-630. |
| [67] | Sun F N, Deng Y X, Ma X S, et al. 2024. Structure-based prediction of protein-protein interaction network in rice. Genet Mol Biol, 47: e20230068. |
| [68] | Szklarczyk D, Kirsch R, Koutrouli M, et al. 2023. The STRING database in 2023:Protein-protein association networks and functional enrichment analyses for any sequenced genome of interest. Nucleic Acids Res, 51(D1): D638-D646. |
| [69] | Virtanen P, Gommers R, Oliphant T E, et al. 2020. SciPy 1.0: Fundamental algorithms for scientific computing in Python. Nat Meth, 17(3): 261-272. |
| [70] | Wang R Y, You X M, Zhang C Y, et al. 2022. An ORFeome of rice E3 ubiquitin ligases for global analysis of the ubiquitination interactome. Genome Biol, 23(1): 154. |
| [71] | Wang X, Li Y, He M Q, et al. 2022. UbiBrowser 2.0: A comprehensive resource for proteome-wide known and predicted ubiquitin ligase/deubiquitinase-substrate interactions in eukaryotic species. Nucleic Acids Res, 50(D1): D719-D728. |
| [72] | Xu C, Wang Y H, Yu Y C, et al. 2012. Degradation of MONOCULM 1 by APC/CTAD1 regulates rice tillering. Nat Commun, 3: 750. |
| [73] | Yang Y, Fu D B, Zhu C M, et al. 2015. The RING-finger ubiquitin ligase HAF1 mediates heading date 1 degradation during photoperiodic flowering in rice. Plant Cell, 27(9): 2455-2468. |
| [74] | Zang G C, Zou H Y, Zhang Y C, et al. 2016. The de-etiolated 1 homolog of Arabidopsis modulates the ABA signaling pathway and ABA biosynthesis in rice. Plant Physiol, 171(2): 1259-1276. |
| [75] | Zeng L R, Park C H, Venu R C, et al. 2008. Classification, expression pattern, and E3 ligase activity assay of rice U-box-containing proteins. Mol Plant, 1(5): 800-815. |
| [76] | Zhu L Y, Cheng H, Peng G Q, et al. 2020. Ubiquitinome profiling reveals the landscape of ubiquitination regulation in rice young panicles. Genom Proteom Bioinform, 18(3): 305-320. |
| [1] | Deng Bowen, Ying Yining, Pan Jianming, Zhang Tongrui, Xu Feifei, Bao Jinsong. Pyruvate Orthophosphate Dikinase B (PPDKB) Deficiency Impairs Starch Biosynthesis and Redirects Carbon Flux to Lipid and Amino Acid Synthesis in Rice [J]. Rice Science, 2026, 33(4): 514-530. |
| [2] | Li Dian, Duan Wenjing, Liu Qun’en, Wu Weixun, Zhan Xiaodeng, Sun Lianping, Zhang Yingxin, Cheng Shihua. Gapless Genome Assembly of ZH8015 and Preliminary Multi-Omics Analysis to Investigate ZH8015’s Responses Against Brown Planthopper Infestation [J]. Rice Science, 2024, 31(3): 317-327. |
| Viewed | ||||||
|
Full text |
|
|||||
|
Abstract |
|
|||||
